Wednesday, September 1, 2021

 Porphyry Copper Deposits

The word “porphyry” is a textural term [not a compositional one] referring to large-grained crystals (called phenocrysts) dispersed in a fine-grained (aphanitic) crystal groundmass. There is commonly a large difference in size between the tiny (can be microscopic) matrix material and the much larger crystals (>2mm). 


The above image is an example of a rock with porphyry texture: a rhyolite (volcanic igneous rock), 12 cm in high. This rock came from a river deposit of Mio-Pliocene age in southern California. This rock does not contain copper.


The next image is an example of pure native copper (50 mm maximum dimension). It was extracted from a porphyry copper rock at a copper mine near Morenci, Greenlee County, Arizona. 


Porphyry copper deposits (PCDs) account for the world’s largest source (about 60%) of copper. These deposits consist of disseminated copper (low to moderate grade [0.3 to 2 percent] copper and copper minerals in vein systems and in fractured rocks (breccias) with porphyry texture and containing copper formed from hydrothermal (heated) fluids that emanated from plug-like magma chambers in the upper crust (less than 5 to 10 km depth). These veins invade host rock, which can range from granitoid  porphyry intrusions (granites to diorites) and from adjacent volcanic wall rocks (rhyolites to basalts). Along with copper, other ores can be associated, like gold, silver, iron, molybdenum, lead, zinc, and tungsten.


The above two views are of the same hand-specimen sample of a copper porphyry from the Keweenaw Peninsula, Michigan, near Lake Superior. The native copper is disseminated in a conglomeratic sandstone/shale interbedded with rift-zone basalt (a volcanic rock). The maximum dimension of this hand specimen is 60 mm.


Porphyry copper deposits have formed throughout most of Earth’s history, but 90 percent of the known ones are Cenozoic or Mesozoic in age. They form mainly in dynamic tectonic areas: under big volcanoes and over suduction zones. They can form, furthermore, in continental magmatic areas along convergent tectonic plate margins or in island-arc environments. PCDs are found predominantly along the west coast of North America (from Alaska to Mexico), the Andes in South America, the Alps region in southern Europe, central Asia, the southwestern Pacific, and the east coast of Australia. 


An example of a continental magmatic area in southwestern North America is the one extending from Nevada to Mexico. An example of an island-arc environment is in Papua (province)  (shown below) is in the southwestern Pacific Ocean area. 


Porphyry copper deposits are currently the largest source of copper ores. Because the content of copper is very low, in many cases the ores are mined via huge open-pit from which massive amounts of rock are excavated and processed. One of the world’s largest and richest PCDs-mines is at Grasberg, Papau, southwest Pacific Ocean. The images below, which are from Google Earth (2020) show the location of this mine, at increasing magnification. In the second image, you can see a road spirally descending into the very large open-pit mine.


The main source of the information I used about PCDs is the very thorough paper by John, D.A., et al. 2010. Porphyry copper deposit model. United States Geological Survey Scientific Investigations Report 2010-5070-B. Chapter B. 169 pp. The pdf is available online for free. 


Thursday, August 19, 2021

Jadeite and Nephrite: the differences

 The purpose of this blog post is to provide some background concerning the generalized word “jade.” It is actually a group name, which “lumps” two different minerals: jadeite and nephrite. Although their chemical properties are different, their physical properties (e.g., hardness, specific gravity [=density], texture, color range, etc.), as well as their geologic origin and setting, can be similar and can overlap. Distinguishing between them is not a trivial matter, especially if you rely on just an “eyeball” identification.” Positive identification requires quantitative mineralogical examination(s). These could include an x-ray diffractometer, infra-red spectrometer, Raman spectrometer, and/or a petrographic microscope study of very thinly cut-and-ground sections of small pieces of the material.

Jadeite and nephrite have a moderate hardness between 6 and 7 on the Mohs Hardness Scale. Yet, they make good ring stones. This is because their aggregate structure makes them extremely tough.


JADEITE


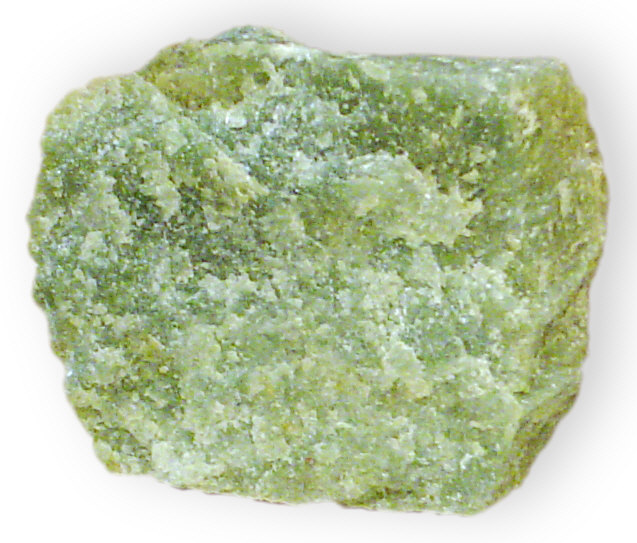
Jadeite is a sodium-aluminium silicate [NaAlSi2O6]. It is a non-hydrous sodic pyroxene mineral. It has monoclinic crystals, a density (specific gravity) of 3.3, and greasy to pearly luster. It is very durable (tough) and difficult to break, but is not all that hard. It has a wide range of colors: apple green to deep green [the most valuable, including the “Imperial jade,” carved in China], shades of blue green, shades of pink and lavender, white (yes! even white) and also black (the rarest). Jadeite is used for making high-end jewelry and artisan pieces. Commercially important original deposits are found in Myanmar (formerly known as Burma), Cuba, Guatemala, Japan, Kazakhstan, Russia, and Turkey.


This is an image of raw jadeite that has not been cut nor polished.

(from Wikipedia 2021).


Jadeite is predominantly found in geologically complex areas called subduction zones, where convergent tectonic plate boundaries, of both modern and ancient continents, collide and where associated high pressures and relatively low temperatures occur inside the Earth’s crust to form metamorphic rocks. These rocks are commonly associated with chemically rich fluids that can partially replace some of the chemical components of jadeite; thus jadeite is rarely pure.


This is a carved piece of jadeite. Image from Wikipedia (2021).


NEPHRITE


Nephrite (Greek, meaning kidney) is a hydrous calcic amphibole silicate mineral with a formula of [Ca(Mg,Fe5Si8O22(OH)2]. It is one of the amphibole silicates. It has monoclinic crystals, a density of 2.96, and greasy to pearly luster. The crystals of nephrite are fibrous and interlock in a very strong matted texture, which is somewhat softer (thus better for carving) than jadeite. Nephrite is closely related to the tremolite-actinolite mineral group and is actually a variant of that group, whose members can be asbestos-like.


This is an ear ring with polished nephrite (7 mm height) in the center. 


Nephrite is more common than jadeite. Nephrite has also a narrower range of colors (mainly green to whitish), and it is used for less expensive jewelry and artisan pieces. Its green color is commonly more subdued and darker than jadeite’s green color. It is found in South Australia, northern British Columbia, China (Xinjiang), Italy, New Zealand, New Zealand, Switzerland, Taiwan, and California.


The image above is a two-ton boulder (slabbed and polished) of nephrite from a placer deposit in south-central Wyoming. The nephrite from this locality ranges from bright green olive and black. This boulder is on display in a stairwell at the Los Angeles County Museum of Natural History.


The aforementioned metamorphic rock/suduction zone geologic setting of jadeite is similar to that of nephrite, except that nephrite forms at lower pressure than does jadeite. Nephrite is known also in placer deposits, which formed by erosion and transport from a host rock and followed by deposition elsewhere in river bottoms, along ocean beaches (California), or in glacial moraines (British Columbia). 


Shown above are two abraded pebbles (largest one with a maximum length of 3 cm) of nephrite from an ocean-beach placer deposit at Jade Cove in Monterey County, California. They have a greasy feel to them.   


NATURAL LOOK-ALIKES


There are many other green minerals that look like jadeite or nephrite. Some are naturally occurring (e.g., emeralds, aventurine, serpentine, olivine, smithsonite, amazonite, green varieties of garnets, etc.).


The image above is a cut-and-polished stone (28 mm height) of aventurine, which is a green microcrystalline form of quartz called chalcedony (see, via the “Search” option at the top of each one of my blogs, for my previous post on “varieties of quartz-part 1”). Although similar in color to jadeite or nephrite, aventurine is very distinctive because it has very tiny, platy mineral inclusions that occur as black dots and streaks.


IMITATIONS OR TREATMENTS 


There is also the possibility that the “jade” you are thinking about buying might be is an imitation (simulant). For example, it might be a piece of green-colored plastic or resin. In some cases, pieces of nephrite have been bleached in acid to remove any unwanted brownish hue, and then stabilized with a polymer. Another possibility is that someone is trying to scam you with dyed-green calcite (= a soft mineral, easily scratched by a knife). 


To protect yourself from fraud, always buy from an absolutely trusted and reputable dealer. If you are still hesitant, you can always consult a gemological association (like the Gemological Association of America or The International Gemological Institution). They use density and/or other definitive mineralogical/petrological tests, and provide you with a copy of the results; just like they do for identification of diamonds versus imitations (see one of my previous posts).

MORE INFORMATION


If you wish to obtain detailed information about jadeite or nephrite, or, for that matter, any other mineral, go to either one or both of the following websites: [note: I consulted them when writing up this blog].


www.gemdat.org


 www.mindat.org


Saturday, August 7, 2021

Crassadoma gigantea: The North American Pacific Coast "Purple-Hinged Rock Scallop"

Scallop bivalves (clams) belong to family Pectinidae, a worldwide group consisting of several hundred species, including some large northern kinds fished commercially for their edible adductor muscle. This muscle, which is used for holding the two valves together, is considered to be a delicacy by many people (Abbott, 1985).

Crassadoma gigantea (J.E. Gray, 1825) is a large scallop living in shallow waters from the Aleutian Islands, Alaska to Bahia Magdalena in Baja California Sur, Mexico. In cooler waters, it reaches its largest size: up to 23 cm in diameter and up to 20 pounds in weight). The name is derived from crassus (Latin: thick) and domus (Latin: house). The common name for this clam is the “purple-hinged rock scallop.” The internal ligament of scallops occupies a triangular pit at the center of the hinge. Crassadoma gigantea is the only species of this genus, which is endemic (confined) to this region. No records of it are known from the Bering Sea, Kamchatka, Japan, or elsewhere.


Crassadoma gigantea has as a fossil record of Miocene to Pleistocene age but only in northern California and Baja California Sur. One of its synonyms of this bivalve is Hinnites giganteus, a name no longer used because it is taxonomically out-of-date.


All of the images shown below are of same specimen (9 cm height and 9 cm width) of C. gigantea from Leo Cabrillo Beach, Los Angeles County, southern California.


                                     Exterior of right valve.


      End view of right valve showing the juvenile-growth region.


The juvenile part of a valve is called the “chlamys” growth stage. A juvenile lives “free” by attaching its strong byssal threads to the substrate. These threads occur on one side of the hinge, and this area (byssal notch) is usually not preserved in the adult stage. The juvenile shell, furthermore, is commonly preserved on both valves. Eventually, the bivalve becomes an adult and becomes permanently cemented to the substrate. Adult Crassadoma gigantea can attach to rock faces or pilings, as well as inside crevices and under boulders. It ranges in depth from intertidal to 80 m.


                                   Interior of right valve.


Exterior of left valve. The white encrustations are of tiny serpulid worm tubes.


                                      Interior of left valve.


Side view of both valves together (articulated), with the right valve (strongly convex) overlying the left valve (nearly flat).


The attached strongly convex right valve, is referred to as the “lower valve,” and the less convex (can be nearly flat) left valve is the “upper valve.” The terms “lower and upper,” however, are relative terms for specimens that commonly attach to vertical surfaces, like steep rock faces or harbor pilings. Permanent attachment to the substrate is rare in pectinids.


Other examples of extant-scallop genera in the world are the pectinids: Pecten, Chlamys, Aequipecten, Amussium, Crytopecten, and Lyropecten. “Wild” scallops have traditionally been harvested using scallop dredges or bottom trawls. In some areas, divers collect the scallops by hand, but this is an expensive process.


On a world-wide basis, in the last few years, there has been a decline in the numbers of “wild” scallop productivity. One reason might be the significant decline in the sharks that prey upon the scallop-eating cownose sting rays. The main diet of these rays is scallops, and without the control offered by the sharks, the sting-ray population is increasing (Milius, 2007; Schmid, 2007).


The simultaneous reduction in sea grasses is another contributing concern. Juvenile scallops (referred to as “spat”) attach themselves to sea grasses before seeking their adult mode of life. Sea grasses provide a sanctuary for the juveniles (Milius, 2007; Schmid, 2007).


Another reason for the decline of “wild” scallop productivity might be the rising acidity of the world’s oceans. At the root of this change is the rising carbon-dioxide levels released into the atmosphere by human activities (pollution) and forest fires. The carbon dioxide is absorbed the oceans, which are showing increasingly higher pH levels. This acidity deprives baby scallops the calcium carbonate they need to grow strong shells. Commercial shell-fishing activities all over the world are at risk, but the Pacific Northwest (especially Washington, British Columbia, and Alaska) are unusually vulnerable because winds that gust south in the summer whip deep water to the surface. These upwellings are even more prone to being acidic, because carbon dioxide tends to be trapped in colder depths (Guilford, 2014).


For more details about C. gigantea, SEE:


Coan, E.V., et al. 2000. Bivalve seashells of western North America. Marine bivalve mollusks from Arctic Alaska to Baja California. Santa Barbara Museum of Natural History Monographs Number 2 Studies in Biodiversity Number 2. 764 pp.


References Cited:


Abbott, R.T. 1985. Seashells of the world. A guide to the better known species. Golden Press, New York. 160 pp.


Guilford, G. 2014. From Our Obsession The Sea. https://qz.com/311345/the-worlds-scallops-and-oysters-are mysteriorly-dying-out/


Milius, S. 2007. Too few jaws: sharks decline let rays overgraze scallops. Science News 171(13):197.


Schmid, R.F. 2007. Shark deaths upset rest of food chain: Shark overfishing may be endangering scallop populations, say scientists. Associated Press/ABC New, May, 29, 2007.


Saturday, July 24, 2021

PART 6 of the Burgess Shale Fossils: 

Pikaia gracilens Walcott (1911, pl. 20, figs. 1. 2) is a legless, soft-bodied, ribbon-like animal, up to 2 inches (5 cm) long, whose closest relatives are the sea-lancelet Branchiostoma and the zebrafish. Although Pikaia was originally thought to be an annelid worm, it is not because it is unsegmented. In the 1970s, its remains were restudied and a notochord was discovered = a rod running along its back and resembling a backbone-like structure. In addition, there are markings on the sides of its body, and they resemble myomeres (chordate muscle bundles) found on living chordates (backboned animals). As a result of this discovery, Pikaia is now classified as probably as a basal, or “stem chordate,” ancestral to all back-boned animals (including fish to humans). In the 1970s, it was reported that Pikaia probably swam like an eel, but, in recent years, researchers have concluded that it was probably a slower swimmer and less flexible than an eel.


Key Reference: 

Walcott, C.D. 1911. Cambrian geology and paleontology. II. No. 5. Middle Cambrian annelids. Smithsonian Miscellaneous Collections. 


Friday, July 9, 2021

 PART 5 of the Burgess Shale Fossils:

Anomalocaris canadensis Whiteaves, 1892 is another part of my discussion on “Middle Cambrian Life: Exceptional Fossils” (Lagerstätt), from the Burgess Shale Member of the Stephen Formation, British Columbia, Canada. Genus Anomalocaris Whiteaves, 1892 ranges from the Middle to Late Cambrian (approximately 505 to 520 million years ago) and has been found at various places, but its principal locality is the Burgess Shale.


Please refer to my earlier post [dealing with the fossil Opabinia] for details about the kit of plastic replicas of some of these fossils, including Anomalocaris canadensis.


Anomalocaris (pronounced “ah-NOM-ah-LO-kar-is”) is a Greek word, meaning "unusual shrimp." Anomalocaris belonged to a group of ancestral arthropods, referred to as “stem-group” of arthropods.


Three views are shown below of a plastic replica of Anomalocaris canadensis: dorsal, side, and ventral, in that order. This replica is 5 inches (12 cm) in length. It is just a fraction of the maximum size of Anomalocaris, which was about 3 (one meter) to 4 feet in length.


Anomalocaris was a soft-bodied, bilaterally symmetrical and flattened animal, with lateral
flaps (attached to gills). Its streamlined body was well designed for swimming. The posterior half of its body was segmented and therefore flexible. On the underside of its body, Anomalocaris had a sturdy mouth, with jaws consisting of numerous plates (oval cones). The mouth was next to two large claws. The body also had two stalked compound eyes, which were advantageous for hunting purposes. 


Anomalocaris was an “apex predator” that probably preferred to eat trilobites.


Determining exactly the type of animal that Anomalocaris represented has a complex history, spanning 100 years! This is because only separate parts of its body were originally found, in a piecemeal fashion, at scattered localities. It was not until workers found enough of these disarticularted parts to finally figure out what the whole animal actually looked like. Thus, each part was described originally as a separate animal. For example, its jaws were described as a jelly fish, and one of its claws was identified as a shrimp. Eventually, a complete specimen was found, and that is when “it all came together.” 


“YouTube” has some really excellent animations about Anomalocaris. I strongly encourage you to “Google them.” They are readily available and extremely easy to use, without any  complicated downloads or troublesome links. Just click on the animations. They are worth watching! 


Saturday, June 26, 2021


PART 4 of Burgess Shale Fossils:

This fourth part of my series about the Early Cambrian fossils of the Burgess Shale in British Columbia, Canada is about Opabinia regalia Walcott, 1912. Wallace found the original material (see first image shown below) and named it. At first glance, it looks like a worm, but the latest interpretation is that this fossil was a member of a “stem group” of phylum Arthropoda (arthro, joint; pod, foot), which is the largest phylum of living organisms. Some modern examples of arthropods are barnacles, crabs, insects, and spiders. Like annelids (worms), the arthropod body is segmented, but in arthropods, there is a fusion and specialization of segments, with two or three major body regions. Opabinia shows some degree of fusion of its segments, thereby indicating a relationship to an arthropod.


Side view of an actual imprint of O. regalia is from Walcott, 1912 (pl. 27, fig. 6). The fossil is about 5.5 cm in length.
 The original reference is Walcott, C.D. 1912. Middle Cambrian Branchiopoda, Malacostraca, Trilobita and Merostomata. Cambrian geology and paleontology, II. Smithsonian Miscellaneous Collection 57:146–228.  

In the images below, I used a plastic model to highlight the anatomical details of Opabinia. Many years ago, one of my graduate students visited a museum gift store, and came across a commercial “kit” with examples of Burgess Shale fossils. The plastic three-dimensional replicas are actually very good, and I used them for teaching purposes in my geology and paleontology classes. Their color schemes are certainly “made up,” but they help to show the dominant anatomical features. I believe that these kits were part of a “limited edition,” thus they are now hard to find. In my previous and subsequent write-ups about some other the Burgess Shale fossils, you will see that I used additional plastic models.


The following images show the dorsal, right side, and ventral views (in that order) of Opabinia regalis, and lastly, a closeup of its five compound (faceted) eyes. Notice the segmented body, numerous legs, tail, fins, and a single (very large) claw. The model shown here is 9.5 cm long, but, as mentioned earlier, the original specimens are up to approximately 5.5 cm in length.


Other Useful References:


Whittington, H.B. 1975. The enigmatic animal Opabinia regalis, Middle Cambrian, Burgess Shale. Philosophical Transactions of the Royal Society of London B, v. 271:1–43.


Briggs, D.E.G. 2015. Extraordinary fossils reveal the nature of Cambrian life: a commentary on Whittington (1975) “The enigmatic animal Opabinia regalis, Middle Cambrian, Burgess Shale, British Columbia. Philosophical Transactions Royal Society B, vol. 370. 


Sunday, June 13, 2021


PART 3 of the Burgess Shale Fossils:

This post is part of a series of six posts dealing with “Middle Cambrian Life: Exceptional Fossils” (Lagerstätt) from the Burgess Shale Member of the Stephen Formation, British Columbia, Canada. Please see my previous two posts; the first of which serves as an introduction to this broad topic.

Wiwaxia corrugata (Matthew, 1899) (new combination) is shown below. There has been considerable controversy about what kind of animal group it represents. It was a soft-bodied, slug-like animal covered in carbonaceous scales and, along its dorsum, with two rows of 7 to 10 blade-like spines. Although some early workers believed that Wiwaxia might be an annelid (worm), that idea has fallen out of favor because Wiwaxia shows no evidence of segmentation. The general consensus is now that Wiwaxia represents a “stem group mollusk” that existed at the time when annelids and mollusks branched off from each other, in an evolutionary sense. Phylum Mollusca (mollusks) is a large group today and consists manily of chitons, scaphopods, bivalves, gastropods, and cephalopods.


The three views below show the bottom (mouth is the "v" shaped structure), top, and side of a plastic replica of Wiwaxia, in that order. The original size of this animal was about 5.5 cm in length.


Some researchers have classified Wiwaxia as a halkieriid, which is a group of Early to Middle Cambrian “small shelly fossils” that consisted of mineralized sclerites, or armored shell plates, which commonly disarticulate upon death. While alive, however, halkieriids looked like slugs in "chain mail."


On its ventral (basal) side, Wiwaxia has a small feeding apparatus consisting of two (rarely three) tooth plates, which are like a mollusk radula (a toothed ribbon of teeth) or the jaws of an annelid.


The name “Wiwaxia” is derived from the Stoney First Nation Nakota language, meaning “windy.” Although, Wiwaxia has been found (mostly as disarticulated scales) at various localities in the world (e.g., China), its principal locality is the Burgess Shale.